Journal of International Research and Reviews
OPEN ACCESS | Volume 2 - Issue 2 - 2026
ISSN No: 3068-370X | Journal DOI: 10.61148/3068-370X/JIRR


Erick Rabiel Kimaro1,2*, Dorice Leonard Lutatenekwa1, and Wilson Charles Wilson3
1Department of Animal, Aquaculture and Range Sciences, Sokoine University of Agriculture
P.O. Box 3004, Chuo Kikuu, Morogoro, Tanzania.
2Tanzania Livestock Research Institute, P. O. Box 202, Dodoma, Tanzania.
3The School of Life Sciences and Bioengineering, Nelson Mandela African Institution of Science and Technology, P.O. Box 447, Arusha, Tanzania.
*Corresponding author: Erick Rabiel Kimaro, Department of Animal, Aquaculture and Range Sciences, Sokoine University of Agriculture
P.O. Box 3004, Chuo Kikuu, Morogoro, Tanzania.
Received: September 20, 2026 | Accepted: September 30, 2026 | Published: October 20, 2026
Citation: Erick R Kimaro, Dorice L Lutatenekwa, and Wilson C Wilson. (2026) “Comparative Assessment of Growth Performance and Nutritional Profile of Panicum Maximum Ecotypes from Diverse Agroecological Zones and Terrains in Tanzania”, Journal of International Research and Reviews, 2(2); DOI: 10.61148/3068-370X/JIRR/024.
Copyright: © 2026. Erick Rabiel Kimaro. This is an open access article distributed under the Creative Commons Attribution License, which permits unrestricted use, distribution, and reproduction in any medium, provided the original work is properly cited.
This study assessed the growth and nutritional value of Panicum maximum ecotypes from two agro-ecological zones of Tanzania (semi-arid and sub-humid) and different terrains (hilly, plain, and valley areas). An on-station experiment was set at Magadu farm at the Sokoine University of Agriculture, involving a complete randomised block design (CRBD) with two blocks and four replicates for assessing the growth and productivity of Panicum maximum under common environmental conditions. Sixteen sprigs from six villages from the two agroecological zones were propagated in a nursery before planting. Sprigs were planted in a randomised plot measuring 2m x 3m, with a consistent inter-plant spacing of 50cm within rows, 60 cm between rows, and 60 cm between adjacent plots within a block. Forage samples from each ecotype were analysed to determine their nutritional composition. The chemical composition analysis included proximate components (Dry Matter (DM), Ash, Crude Protein (CP), and Crude Fiber (CF)) and fibre fractions (Neutral Detergent Fibre and Acid Detergent Fibre). The statistical differences in nutritional traits were tested using a two-way ANOVA at p<0.05. The results showed that plant height was significantly higher for the ecotypes from the semi-arid zone (201.64 cm) compared to the ecotypes from the sub-humid zone (99.83 cm; p < 0.0001). Among ecotypes, significant differences were observed for leaf width and fresh weight, with valley ecotypes having the widest leaves (2.65 cm) and the highest forage fresh weight (12.23 kg), while plain-area ecotypes recorded the narrowest leaves (1.79 cm) and the lowest forage fresh weight (8.04 kg). Moreover, significant interaction was observed between zones and terrains for leaf to stem ratio (p = 0.047), leaf width (p = 0.046), and fresh weight (p = 0.022), indicating that the response of these traits varied across zones and terrains. Ecotype significantly influenced ash, crude protein and dry matter content, with plain-area ecotypes showing the highest crude protein (5.42%) and dry matter (36.20%), while hilly and valley ecotypes had higher ash content. These results demonstrate the adaptive variability of Panicum maximum ecotypes and highlight the importance of selecting agroecological zone-specific ecotypes to optimize forage yield and nutritional quality across diverse Tanzanian environments.
Biomass, hill, plain, valley & zones
Livestock production is one of the key components of Tanzania’s agricultural sector, contributing significantly to rural livelihoods and national food security (Suleiman 2018). However, ruminant productivity, especially that of cattle, sheep and goats, remains low in most production systems due to factors such as limited feed resources, poor nutritional quality of feed and environmental constraints (Capper & Bauman 2013; Burkart et al 2024). Animal growth, reproduction and milk production are severely constrained by seasonal feed shortages during the dry season (Rustis et al 2023).
The continuing deterioration of Tanzania's rangelands is significantly related to the problem of forage scarcity (Sangeda & Maleko 2018). Research shows that most of the nation's rangelands experience decreased grazing capacity, increased bare ground and decreased vegetation cover. For instance, a recent study by Wiethase et al (2023) shows that the rangeland ecosystems in northern Tanzania have lost their ecological resistance as a result of ongoing overgrazing, soil erosion and frequent drought. Another study conducted in eastern Tanzania indicated lower-quality forage due to a significant decline in herbaceous vegetation, particularly palatable grasses (Maro et al 2021). These patterns demonstrate that rangeland degradation remains a significant barrier to sustainable livestock production in Tanzania (Mussa et al 2016).
Tanzania has abundant forage species well adapted to diverse agroecological zones. However, most drought tolerant native grass species in the country are underutilised and poorly conserved (Masao et al 2023). One of the main ways to reduce the country's feed deficit is to support native forage species and strengthen forage seed systems (Burkart & Mwendia 2024). However, Tanzania's current forage seed system is still inadequate, as evidenced by the country's reliance on unofficial channels, limited seed availability, and poor multiplication of locally adapted varieties (Ngunga & Mwendia, 2020). As a result, few suitable forage species have been adopted and promoted for rangeland rehabilitation (Ngunga & Mwendia 2020).
Panicum maximum is a native grass to Tanzania, and was selected for this study due to reported traits of adaptability, biomass production and overall performance (Lievio et al 2025). According to Homewood et al (2009), Panicum maximum's deep and dense root system allows it to withstand fire, drought and poor soils, while in the right circumstances it yields a significant amount of fodder. Its adaptability across a variety of agro-ecological zones, including semi-arid and sub-humid regions where it maintains stable biomass production and shows significant morphological variation linked to local environmental factors, has been further confirmed by studies conducted by Genetic et al (2021) and Benabderrahim & Elfalleh (2021).
The importance of systematic ecotype evaluation and targeted multiplication of superior forages is reinforced by regional and international studies outside of Tanzania (Namazzi et al 2020; Gouveia et al 2021 and Silveira et al 2025).. Multi-genotype trials and germplasm characterisations have been employed to identify high-performing forage ecotypes in East Africa (Kirwa E C 2019). For instance, Napier grass genotype trials has been conducted in Ethiopia, and has shown notable genotype × environment variations in biomass yield and adaptation (Rustis et al 2023). Similarly, assessments of Brachiaria ecotypes in Uganda have shown a high level of genetic diversity and unique gene pools that could be used for selection and conservation (Namazzi et al 2020). Moreover, warm-season grasses, like Paspalum vaginatum, have undergone international multi-environment and shade tolerance trials that show how coordinated evaluation across environments identifies ecotypes with stable performance and stress tolerance (Gouveia et al 2021) & (González Marcillo et al 2021).
The justification for similar ecotype assessments of Panicum maximum in Tanzania is supported by the collective findings of East African and international studies (Kabirizi et al 2013; Khan et al 2015). These studies demonstrate that evaluating multiple ecotypes under specific conditions consistently reveals superior forage ecotypes for multiplication and deployment. Regarding this body of work, there remains a gap in Tanzania; where relatively few studies have directly compared multiple forage ecotypes under a common environment (Lutatenekwa et al 2021). Growth, regrowth, dry-matter production, nutritional value and persistence traits are all important for selection and multiplication, which can be measured in a controlled environment.
Significant genetic and phenotypic variation exists among Panicum maximum ecotypes, affecting characteristics like drought tolerance, biomass accumulation, tillering capacity, drought and disease persistence (Pessoa-filho et al 2021). Moreover, genetic diversity among accessions gathered from various environments is highlighted by molecular characterisation studies, suggesting the possibility of choosing drought-resistant and productive ecotypes (Jiang et al 2022); (Obayelu A. E 2023). This variation emphasises the importance of testing several ecotypes in consistent conditions to evaluate their performance objectively.
The present study aimed to identify P. maximum ecotypes with superior agronomic traits that are appropriate for large-scale multiplication and use in rangeland restoration by evaluating the growth performance, yield and nutritional quality of various Panicum maximum ecotypes under common environmental conditions. This objective is in line with recommendations from recent studies on rangeland restoration, which demonstrate that degraded rangelands can recover with proper management and reseeding with resilient grasses (Wiethase et al 2023; Leger et al 2021) and (Sangeda & Malole 2014). By choosing and expanding high-performing ecotypes, Tanzanian livestock productivity will be increased by improving the supply of forage for ruminants, supporting the rehabilitation of degraded rangelands and increasing the availability of adapted forage planting materials. Therefore, this study will play an important role to mitigate challenge of forage availability in Tanzania rangelands, especially during the dry season.
Materials and methods
Description of the Study Area
This study was conducted at Magadu farm located at the Edward Moringe Campus of Sokoine University of Agriculture (SUA) in Morogoro Municipality, Eastern Tanzania. The farm is located between 500 and 600 meters above sea level, on the lower slopes of the Uluguru Mountains, about 195 kilometres west of Dar es Salaam. The topography of the area is characterised by flat flood plains, and a generally level landscape with gentle slopes, with bimodal rainfall pattern and receives between 500 and 1800 millimetres of rainfall annually. The heaviest rains usually fall in March and April during the extended rainy season, which runs from late February to the end of May. From November through January, there are brief rains. Moreover, rainfall distribution can be irregular despite this bimodal pattern, which can occasionally cause moisture stress, especially for rain-fed crops like maize. The tropical climate of Magadu Farms is also reflected in temperature patterns. Temperatures during the day typically range from 27 to 31 °C, creating warm conditions that are ideal for raising livestock and crops. The temperature at night may fall to about 14 °C during the coldest months.
Source, collection and multiplication of experimental materials
The study involved the systematic collection of 16 sprigs of Panicum maximum from two agro-ecological zones of Tanzania (semi-arid areas of Mpwapwa district in Dodoma region and sub-humid areas of Moshi rural district in Kilimanjaro) and different terrains (hilly, plain, and valley areas). One ward was selected from each district. From each ward three villages were purposively sampled based on their differences in agro-ecological characteristics, topography, significant potential in ruminant’s production and presence of Panicum maximum. This was based on the preliminary survey and consultation with the respective district extension offices (Kimaro et al 2025). The procedures used for selecting the sites for sprigs collection, as described above were based on the reference study by De Glanville et al (2020). Mpwapwa ward was selected from Mpwapwa district and Marangu ward from Moshi rural district. Three villages sampled from Mpwapwa include Kikombo, Ilolo and Chibwechangula representing ecotypes from hill areas, plain areas and valley areas, respectively. Villages from Marangu ward included Mbahe kati, Mkuuni and Kileo representing ecotypes from hill areas, plain areas and valley areas, respectively.
Sprigs were handled carefully using plastic bottles contained with moisten soil to avoid desiccation. A nursery was prepared adjacent to the experimental site to hold the sprigs and facilitate propagation before planting. Sprigs from the same village were planted together in the same row, with an inter-row spacing of 1 meter and 50 cm between individual sprigs. Following propagule multiplication, an adequate number of sprigs were available to facilitate the experiment (Peterson et al 2010); (Sena 2021).
Experimental design and treatments
An experiment was set at SUA, Magadu farm, in a complete randomised block design (CRBD) with two blocks, and each block consisted of four replicates for assessing the growth and productivity of Panicum maximum under common environmental conditions. Experiment was done for 90 days from 19th May, 2025 to 18th August, 2025. Irrigation was applied early morning every two days equally on each plot. The experiment consisted of two blocks; Block one comprised 16 plots measuring 3 × 2 m planted with sprigs of Panicum maximum sourced from semi-arid areas and a control. Block two also comprised 16 plots of 3 × 2 m and was planted with sprigs of Panicum maximum from a sub-humid area and a control. In total, the experiment includes 32 plots. Each plot in both blocks was planted with 15 sprigs of Panicum maximum, spaced 50 cm apart. Sprigs were planted randomly into a 2m by 3m plot, maintaining a space of 50cm between plants and 60cm between rows. Inter-plot spacing was set at 60 cm, with a 2m separation between blocks.
Data Collection
Parameters Measured and Procedure
The parameters assessed during data collection were sprouting date, days at first flowering, 50% flowering, full flowering, days to maturity, stem height, leaf to stem ratio (L-S ration), leaf length, leaf width, net plot fresh weight, net plot dry weight, and a sample of forage from each ecotype were taken to laboratory for proximate analysis to determine their nutritional composition. The height of the plant was measured in centimetres (cm) from the base of the stem (at the soil’s surface) to the highest point of the plant using a tape measure (Adnew et al 2022). The length of the leaf was measured from the apex of the blade to the base of the petiole, and the width was measured at the widest point perpendicular to the longitudinal axis of the leaf (Schrader et al 2021). Leaf-to-stem ratios were done by selecting three healthy tussocks at the centre of each plot, and the number of leaves was counted. The average was then calculated to obtain the mean leaf to stem ratio (Mganga et al 2021).
Flowering time was recorded at three stages: onset of flowering (first flowering), 50% flowering, and full (100%) flowering. Full flowering across most forage ecotypes occurred after 75 days, though some required up to 80 days Flowering time is frequently targeted in breeding programs because flowering time has a strong correlation with potential yield (Iannucci et al 2008). Fresh weight was determined at maturity 80 days post planting. All forage within each plot was harvested using a sickle and weighed to estimate productivity. Subsequently, a 500gm sample was collected from each plot for proximate analysis to determine nutrient composition.
Data Analysis
Laboratory Analysis
Three samples of 500grams fresh forage from each ecotype were collected from the experimental plots and placed in clean, labelled polyethylene bags. To reduce moisture loss and biochemical alterations, the samples were transported to the laboratory as soon as they were collected. Upon arrival, the fresh samples were oven-dried at 60–65 °C until they reached a constant weight to ensure total moisture removal and prevent nutrient degradation. The dried samples were then allowed to cool at room temperature in a desiccator for 10 minutes. Samples were ground for passage through a 1mm sieve after being oven dried at 60 to 65 °C to constant weight. Before analysis, ground samples were mixed thoroughly and kept in air-tight containers. Proximate composition was determined by using Near Infrared Reflectance Spectroscopy (NIRS) at the Tanzania Veterinary Laboratory Agency (TVLA). Samples were scanned using the near infrared range of 780 to 2500 nm, and reflectance spectra were analysed using calibration models developed from the standard wet chemistry reference data. The calibrated model was used to predict the proximate composition of forage samples, including moisture content, crude protein, crude fibre, ether extract and ash content (Serpa-imbett et al 2025). Dry matter content was calculated using the following formula:
Dry Matter DM%=Dry Weigh of Sample (DW)Fresh Weigh of Sample (FW)X100%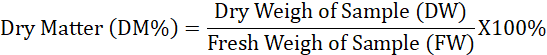
Whereby: Fresh weight (FW) = Weight of a sample before drying
Dry weight (DW) = Weight of a sample after oven drying to a constant weight.
Data Processing and Statistical Analysis
Data analysis was conducted using the General Linear Model (GLM) procedure in SPSS (version 25). Prior to analysis, data distribution was assessed using the Shapiro-Wilk test. Then, a two-way ANOVA test was performed to test a significant difference at p<0.05. The ecotypes from different terrains and zones were treated as fixed effects (independent variables). Pairwise comparisons were evaluated using the least square difference (LSD) test at a significance level of p < 0.05. Least square means (LSMs) were computed for all variables. The statistical model is as in equation 1 below:
Yij = μ + Zi +Tj + (Zi*Tj) + eij. …………………………………………………....…………. (1)
Where;
Yij = Response (morphological chrematistics and nutritional status) of P. maximum of the ith zone and jth terrain,
μ = Overall mean effect
Zi = Effect due to different zones
Tj = Effect of ecotype from different terrains
Zi*Tj = Effect of interaction of zone and ecotypes from different terrains
Eij = Error term.
Results
Growth performance and yield of Panicum maximum ecotypes from two different agro-ecological zones in Tanzania
The results revealed that the growth performance of Panicum maximum ecotypes differed significantly between the two agro-ecological zones (p<0.05), as shown in Table 1 below. The plant height was significantly greater (p < 0.0001) in the semi-arid (SA) zone of Mpwapwa (201.64 cm) compared to the semi-humid (SH) zone of Moshi (99.83 cm). Although leaf–stem ratio (L–S ratio) and tiller number did not differ significantly between zones (p > 0.05), plants from Mpwapwa showed slightly higher values.
Based on terrains, plant height, L–S ratio, tiller number, leaf length, fresh weight, dry weight, and dry matter percentage did not differ significantly (p > 0.05) among the ecotypes, except for leaf width (p = 0.025) and fresh weight (p = 0.042). The valley ecotype (VA) exhibited the widest leaves (2.65 cm) and the highest fresh biomass (12.23 kg), while the plain area ecotype (PA) had the lowest fresh weight (8.04 kg). Significant zone × ecotype interactions (Figure 1) were observed for L–S ratio (p = 0.047), leaf width (p = 0.046), and fresh weight (p = 0.022), indicating that the response of these traits varied across terrains/environments.
Table 1: Growth performance and Yield Parameters of different Panicum maximum ecotypes from two different agro-ecological zones in Tanzania
|
Factor |
Category |
Plant height |
L-S ratio |
Tiller number |
Leaf length |
Leaf width |
Fresh weight |
Dry weight |
DM |
|
Zone |
Moshi (SH) |
99.8b |
8.17 |
8.5 |
52.7 |
2.11 |
9.05 |
4.72 |
50.4 |
|
|
Mpwapwa (SA) |
202a |
9.28 |
15.3 |
49.8 |
2.31 |
11.1 |
5.24 |
45.9 |
|
Ecotype |
Hilly area (HA) |
146 |
9.04 |
10.2 |
50.4 |
1.79b |
10.0ab |
4.69 |
46.6 |
|
|
Plain area (PA) |
147 |
9.25 |
10 |
52.4 |
2.19ab |
8.04b |
3.8 |
45.6 |
|
|
Valley area (VA) |
158 |
7.88 |
15.6 |
51.0 |
2.65a |
12.2a |
6.45 |
52.2 |
|
|
SEM |
12.6 |
0.52 |
3.81 |
6.18 |
0.17 |
0.92 |
0.76 |
4.75 |
|
|
P-values – Zone |
<0.01* |
0.12 |
0.18 |
0.72 |
0.36 |
0.09 |
0.59 |
0.55 |
|
|
P-values – Ecotype |
0.85 |
0.29 |
0.65 |
0.97 |
0.03* |
0.04* |
0.14 |
0.37 |
|
|
P-values – Zone × Ecotype |
0.54 |
0.05* |
0.69 |
0.91 |
0.05* |
0.02* |
0.12 |
0.33 |
NU
Nutritional status of Panicum maximum from different terrains of two selected agro-ecological zones in Tanzania.
The estimated marginal means of the nutritional composition of Panicum maximum ecotypes across the two agro-ecological zones are presented in Table 2. Agro-ecological zone significantly influenced acid detergent fibre (ADF), neutral detergent fibre (NDF), ash and dry matter (DM) contents (P < 0.05), but had no significant effect on crude fibre (CF) and crude protein (CP) content. Grasses from the semi-arid zone (Mpwapwa) recorded significantly higher ADF than those from the semi-humid zone (Moshi). In contrast, ash and DM contents were significantly higher in the semi-humid zone compared with the semi-arid zone.
Ecotype significantly affected ash, CP and DM contents (P < 0.0001), while no significant differences were observed for ADF and CF. The hilly area ecotype had the highest ash content, whereas the plain and valley ecotypes showed lower ash values. Crude protein content was highest in the plain area ecotype and lowest in the hilly and valley ecotypes. Similarly, dry matter content was significantly higher in the plain area ecotype compared with the hilly and valley ecotypes. A significant interaction between zone and ecotype was observed for all measured nutritional parameters (P < 0.05), indicating that the response of Panicum maximum ecotypes in terms of ADF, Ash, CF, CP and DM varied depending on the agro-ecological zone (Figure 2). This suggests that both environmental conditions and ecotype characteristics jointly influence the nutritional quality of P. maximum.
Table 2: Means of nutritional status of Panicum maximum ecotypes from two agro-ecological zones
SH=Sub-humid zone, SA= Semi-arid zone, HA=Hilly area, PA=Plain area, VA=Valey area, SEM=Standard error of the mean, ADF=Acid detergent fibre, CF=crude fibre, CP=Crude protein, DM=dry matter.
Discussion
The optimization of livestock production system in Tanzania is fundamentally linked to the availability of high-quality adaptable forage species. As Panicum maximum remains a cornerstone of the tropical emotional grazing. Understanding the variability in growth performance and forage nutritional quality of P. maximum across different agroecological zones and terrains is essential for optimising its utilisation in livestock production systems. The present study examined the growth traits and nutritional quality of Panicum maximum ecotypes grown in varied agroecological zones and terrains in Tanzania. By assessing these variables in controlled experimental settings, the study aimed to pinpoint ecotypes that are best suited to specific environments, thereby promoting forage production and increased livestock productivity across diverse agroecological zones and terrains of Tanzania, as further discussed below.
Growth characteristics and yield of Panicum maximum ecotypes from two different agro-ecological zones in Tanzania
The present study reveals a significantly taller plants in Mpwapwa (semi-arid zone) compared to Moshi (sub-humid zone) demonstrating a strong environmental influence on the vegetative growth of Panicum maximum. This finding aligns with the study of Kisambo et al (2022), which reported enhanced stem elongation and plant height of Panicum maximum under moisture-limited conditions (Kisambo et al 2022), attributing this response to adaptive strategies aimed at optimizing light interception and persistence under stress, a mechanism consistent with the taller growth observed in Mpwapwa. Semi-arid conditions often favour vertical growth as grasses allocate resources toward height rather than lateral expansion, improving competitiveness under limited soil moisture and grazing pressure. In contrast, the relatively shorter plants in Moshi suggest that sub-humid environments promote more balanced vegetative development. Similar observations were reported by Okwori and Abdulsalam (2017), who found that forage grasses grown under moderate rainfall exhibited reduced height but improved canopy uniformity. This supports the notion that Panicum maximum adjusts its architecture according to moisture availability, balancing height and leaf development in more favourable environments (Malaviya et al 2020).
The absence of significant agro-ecological zone effects on leaf length, leaf width, biomass components and dry matter percentage indicates a high degree of morphological stability of Panicum maximum across contrasting environments. This stability concurs with findings from the Nigerian savannah study, which showed that several forage grass species, including Panicum maximum, maintained consistent leaf and yield traits across locations (Araujo et al 2018). Key factors that influence for the seasonal production of Guinea grass. Scientia Agricola, 75(3), 191-196. Such plasticity suggests that Panicum maximum possesses adaptive traits that allow it to sustain forage quality and productivity across diverse ecological conditions.
Our findings revealed that dry matter percentage did not differ significantly between zones, implying similar tissue composition regardless of moisture regime. This observation is particularly important for forage utilization and is consistent with results from the study by Kisambo et al (2022), where dry matter content of Panicum maximum ecotypes remained stable across environmental treatments. Moreover, recent studies show that stable dry matter accumulation ensures reliable forage quality, making Panicum maximum suitable for use in both semi-arid and sub-humid systems (Province et al 2021).
Variation among terrain ecotypes revealed a significant effect on leaf width, with the valley ecotype (VA) exhibiting the widest leaves. This trait is likely linked to enhanced moisture availability and soil fertility in valley environments, promoting leaf expansion. Similar genetic and morphological variation among P. maximum genotypes was documented in the study of Roy et al (2021), which identified leaf width as a key discriminating trait among ecotypes. Wider leaves were associated with higher photosynthetic capacity and biomass accumulation, supporting the superior performance of the valley ecotype observed in the present study.
Fresh biomass yields also differed significantly among terrain ecotypes, with the valley ecotype producing the highest fresh weight (12.23 kg). This agrees with findings from both the Nigerian savannah study and the germplasm diversity analysis, which reported that genotypes adapted to favourable micro-environments consistently produced higher fresh biomass (Omokanye & Onifade 2000). However, the lack of significant differences in dry weight suggests that fresh weight variation may be influenced by higher moisture content rather than greater structural biomass accumulation, a pattern also noted in the simulated grazing experiment (Aganga et al 2003).
The significant interactions between agro-ecological zone and terrain for leaf–stem ratio, leaf width and fresh weight revealed in the present study indicate differential ecotype responses depending on environmental conditions. These interaction effects reinforce conclusions in line with the findings from Roy et al (2021), which emphasized the importance of matching genotype performance to specific environments. Ecotypes performing well in valley conditions may not necessarily exhibit similar advantages under semi-arid or sub-humid zones, highlighting the need for environment-specific ecotype selection in forage improvement programs. Overall, the findings demonstrate that while agro-ecological conditions primarily influence plant height, terrain-based ecotypic variation plays a major role in shaping leaf traits and fresh biomass production. The superior performance of the valley ecotype under favourable conditions and the stable growth of other ecotypes across zones reflect the broad adaptability of Panicum maximum. These results are consistent with previous studies and confirm the species’ morphological resilience and suitability for diverse production systems across Tanzania and similar agro-ecological regions.
Nutritional status of Panicum maximum from different terrains of two selected agro-ecological zones in Tanzania
The observed variation in the nutritional composition of Panicum maximum across agro-ecological zones and terrain types underscores the strong influence of environmental conditions, terrain-related factors and ecotypic adaptation on forage quality. The significantly higher ADF content recorded in the semi-arid zone (Mpwapwa) compared with the sub-humid zone (Moshi) suggests greater accumulation of structural carbohydrates under moisture-limited conditions. This pattern is consistent with findings by Kisambo et al (2022), who reported that Panicum maximum ecotypes in semi-arid environments tend to invest more in cell wall components as an adaptive strategy to drought stress and grazing pressure. Similar observations have been reported in other tropical grasses, where water stress promotes lignification and fibre deposition, thereby reducing digestibility (Minson 1990; Van Soest 1994). However, some studies have shown that adaptive management, such as earlier harvesting or fertilization, can mitigate fibre accumulation even under semi-arid conditions (Humphreys 1991), suggesting that management interventions may partially offset environmental constraints.
In addition, higher NDF recorded in Moshi (19.41%), indicated that greater fiber accumulation under relatively favorable conditions, which may reduce forage intake. Among ecotypes, the plain area showed the highest NDF (19.46%), followed by the valley (18.65%) and the hilly (17.88%), suggesting variability in cell wall content due to genetic differences. The significant zone × ecotype interaction further indicates that NDF response depends on environmental conditions. Similar variations in fiber fractions across environments and genotypes have been reported by Adnew (2022) and de Araujo et al (2018).
In contrast, the higher ash and dry matter contents observed in the semi-humid zone likely reflect improved soil moisture availability and nutrient uptake, which enhance mineral accumulation and biomass production. These findings align with Okwori and Abdulsalam (2017), who reported superior mineral content and overall forage quality of guinea grass grown under more favourable climatic conditions in the Southern Guinea Savannah of Nigeria. Similarly, Skerman and Riveros (1990) noted that guinea grass grown in higher rainfall areas tends to exhibit improved mineral nutrition and herbage yield. However, contrary evidence has been reported by Mahala et al (2015), who found that excessive rainfall can sometimes dilute mineral concentrations in forage due to rapid biomass accumulation, indicating that the relationship between moisture availability and ash content may not always be linear.
Differences among ecotypes further emphasise the role of terrain-related adaptation in influencing nutritional quality. The higher ash content observed in the hilly area ecotype may be attributed to soil erosion and nutrient redistribution commonly associated with sloping landscapes, which can concentrate certain minerals in plant tissues. Comparable results were reported by Mtengeti et al (2008), who observed higher mineral content in forages growing on upland terrains in eastern Africa. Conversely, the superior crude protein and dry matter contents recorded in the plain area ecotype suggest more favourable growing conditions, such as deeper soils, reduced erosion and better moisture retention. Roy et al (2021) reported substantial genetic diversity among Megathyrsus maximus genotypes, particularly for biomass production and nutritional traits, supporting the view that inherent genetic differences among ecotypes strongly influence forage performance across varying environments. In contrast, Adjei et al (1988) found minimal differences in crude protein among guinea grass ecotypes grown under uniform management, suggesting that environmental effects may outweigh genetic effects under certain conditions.
The significant interaction observed between zones and ecotype for all nutritional parameters highlights the combined influence of genotype and environment on forage quality. This interaction implies that the nutritional performance of a given Panicum maximum ecotype cannot be generalised across environments, as trait expression is highly context-dependent. Kisambo et al (2022) similarly emphasised that guinea grass ecotype performance varies with climatic conditions and grazing management. Comparable genotype and environment interactions have also been reported by Roy et al (2021) and Boonman (1993), who demonstrated that forage quality traits respond differently across ecological gradients. However, some studies have suggested relatively stable performance of certain improved guinea grass cultivars across environments (Hare et al 2013), indicating that selected genotypes with broad adaptability may reduce environmental variability in forage quality. These results indicate that both agro-ecological zone and terrain play critical roles in shaping the nutritional status of Panicum maximum in Tanzania. Strategic selection and deployment of ecotypes suited to specific environments, particularly plain-area ecotypes for improved crude protein and dry matter yield, could enhance forage quality and livestock productivity.
Conclusion and recommendations
The results demonstrate that the environment plays a major role in plant height, while ecotype terrain influences leaf traits and fresh biomass production of Panicum maximum. The strong performance of the valley ecotype suggests that it is more productive under favourable conditions, while the stability of other ecotypes across zones indicates adaptability. Moreover, the findings show that agro-ecological zone and terrain significantly influence the nutritional quality of Panicum maximum in Tanzania and selecting ecotypes adapted to specific environments, especially plain-area ecotypes, can improve crude protein, dry matter yield and overall forage value. Therefore, the morphological and nutritional stabilities across different terrains highlight the resilience of Panicum maximum in diverse Tanzanian environments. The study suggests that targeted ecotype selection remains important for maximising forage yield in specific zones.
Acknowledgement
I sincerely thank Sokoine University of Agriculture (SUA), particularly the Department of Animal, Aquaculture and Range Sciences, for their continuous guidance, support, and close follow-up throughout the research activities. I also express my sincere gratitude to the Tanzania Livestock Research Institute (TALIRI) for granting me study leave to pursue my Master's degree, which made this research possible.
Open Access By Aditum Open Access Journals id licensed under Creative Commons Attribution 4.0 International License. Based On a Work at aditum.org


